

Blog Archive:
Beneath Our Feet

Soil Carbon Modelling with Soil Fauna and Humus Forms
By Cindy H. Shaw, Oleg Chertov, and Darrell Hoffman*

An example of a mull humus form.
Image by D.Hoffman
Soil fauna are key agents in different types of organic debris processing in the forest floor and mineral topsoil, resulting in humus forms. The humus form that develops at any given site is the result of the amounts and types of litter inputs (such as wood, leaves, roots) from local vegetation, temperature and moisture conditions, and the dynamics of soil biota including fauna, fungi, and bacteria. Humus forms are most broadly divided into three orders: mor, moder, and mull. Each order is associated with a set of physical properties that are easily observed and are related to processes occurring in the forest floor and the underlying mineral soil.

An example of a moder humus form.
Image by C.McNalty
Mors are characterized by a distinct boundary between organic and mineral soil horizons, often with plentiful plant roots and fungal hyphae throughout the organic layers. Mulls develop when there is sufficient mixing of organic and mineral soil often resulting from the activities of soil fauna; they have a relatively thick, dark, mineral Ah horizon enriched with organic matter.
Moders are humus forms with properties that transition between those of mors and mulls. The orders can be further divided into groups described by horizon types (such as L, F, H, Ah), which indicate the stage of decomposition, or include descriptors for composition (such as woody, fungal mossy).
The activities of different organisms and the interactions among them have direct consequences for carbon dynamics, as they are the agents driving rates of mineralization and respiration, as well as stabilization, and sequestration. Although the actions of soil fauna mediate the cycling and storage of carbon, the direct effects of these organisms can be difficult to study, and until now have not been included in carbon models. In addition, most carbon models focus on predicting carbon emissions because of the great interest in greenhouse gases, and they neglect the formation and storage of soil organic matter, which is important in carbon sequestration.

An example of a fungal mor humus form.
Image by C.McNalty

An example of a woody mor humus form.
Image by C.McNalty
Recently, a model developed by scientists in Russia, Germany and Canada, Romul_Hum (the soil module of the individual tree forest growth model EFIMOD), integrates knowledge of humus form development, soil fauna food webs, dynamics of fungi and bacteria, and the resultant formation and stabilization of carbon in soil organic matter. Romul_Hum accounts for the many belowground interactions (fungivory, bactivory, predator-prey relationships) between soil fauna, bacteria, and fungi and how these interactions are regulated by the qualities of incoming vegetative material. Unlike other models, which treat decomposers as a homogenous group, Romul_Hum uses variations in the ratios of fungal to bacterial biomass, and the ratios of carbon to nitrogen in the fungal and bacterial biomass. Based on published soil fauna data, different types of food webs are defined for combinations of decomposers and types of horizons in humus forms. An earthworm module was developed with parameters for for food palatability, ingestion and egestion, food consumption, lifespan, excretion, and assimilation efficiency. It is especially important to understand the effects of earthworms interacting with other soil fauna activities in Canada as earthworms are invasive to Canada’s large boreal forest (see blog: Earthworm invasions in northern forests). As earthworms spread through the Canadian boreal forest, they will change the carbon dynamics and carbon balance of the ecosystems.

An invasive earthworm and lepidoptera larva in a boreal forest soil sample.
Image by C.McNalty
Romul_Hum could be used to predict, understand, and quantify those changes. The types of changes to the forest carbon cycle from invasive earthworms is dependent on the species of earthworm(s) present. These changes can include mixing organic material in the forest floor with the mineral soil below, shifting the balance between fungal and bacterial biomass, and stabilizing carbon in soil organic matter as it moves through the gut of the earthworm, or as earthworms ingest and stabilize faeces produced by meso-fauna. Beyond these effects, earthworms can change the food and habitat available for other groups of soil fauna, such as nematodes, mites, and springtails, affecting the survival and success of meso-faunal populations.

The Forest Floor Recovery Index
Image by D.Hoffman
By acknowledging and accounting for the complex interactions between soil faunal food webs and their habitat (humus forms), the modelling approach of Romul_Hum provides a means to evaluate how management, and potentially climate change, affects relationships between soil fauna biodiversity and soil carbon sequestration. In Europe, humus form classification is currently being refined within the HUMUSICA project. In Canada, humus forms are used as part of a system (Forest Floor Recovery Index) to evaluate the success of reclamation after mining.
*Cindy Shaw (cindy.shaw@canada.ca(link sends e-mail)) is a Research Scientist, and Darrell Hoffman (darrell.hoffman@canada.ca(link sends e-mail)) is a Forest Soil Research Assistant, for the Canadian Forest Service at Natural Resources Canada. Oleg Chertov is a scientist who has worked in Russia, Germany, and Finland, and created the Romul_Hum models with Alex Komarov

Romul_Hum predictions of soil carbon stocks and their distribution between the mineral Ah and organic O horizons, depending on presence of mesofauna and
earthworms.
Image by O.Chertov

Assessing Amazonia Biodiversity: Beyond the Taxonomic Impediment
By Camila Ritter, PhD. student, University of Gothenburg

Amazonia is the largest tropical rainforest with the highest level of species diversity in the world. However, most of what is known about patterns of biodiversity in this area is based on large-sized and well-studied organisms such as mammals, birds, amphibians, and flowering plants. Because these macro-organisms constitute just a small fraction of the world’s total biodiversity (vertebrates represent only about 0.7% of all species of eukaryotes, for instance), and no consensus has been reached on whether poorly studied taxonomic groups such as arthropods and micro-organisms follow the same distribution patterns as macro-organisms, it is urgent to put more efforts in this ‘hidden’ biodiversity.
However, to achieve this goal we must overcome a severe obstacle: the so-called taxonomic impediment. Considering that it takes, on average, 21 years from the first collection of a species until its formal description, we would have to wait another 1,200 years to catalogue all extant species. That is unacceptably slow, and we need to develop and validate new methods for faster, more cost-effective, and objective biodiversity assessments, which do not rely on manual identification of specimens. Fortunately, molecular tools have opened a new research window on biodiversity through genetic data. With methods such as metabarcoding, it is now possible to quantify phylogenetic diversity of any locality without the need for a priori classification of specimens.
In an effort to assess the main patterns of biodiversity distribution in Amazonia, we have sequenced genetic markers from both prokaryotes and eukaryotes from a range of soil and litter samples. We targeted four locations covering the different kinds of habitat (tropical rainforest, seasonal flooded forests, and naturally open areas) of the Amazonia. If we find that environmental genetic diversity and traditional taxonomic metrics are highly correlated, that would mean that biodiversity can be rapidly and cost-effectively assessed without the demand of taxonomic experts. This result would facilitate the detection and protection of areas of high biodiversity and would allow taxonomists to focus on species descriptions and the biology of the underlying organisms, rather than routine specimen identifications. If these variables, however, are found not to be correlated, it would mean that despite centuries of research we still know virtually nothing about how the great majority of the world’s biodiversity is distributed.

Naturally open area on Amazonia. These areas have an insular distribution in “seas” of tropical forest and are associated with white sand soil. This picture was taken on “Reserva da Campina”, close to Manaus, AM, Brazil.
Photo credit C.Ritter

The tree shows the water mark from flood season of Várzea, seasonally flooded forest.The mark indicates a flood height of around 15 meters.
Photo credit C.Ritter
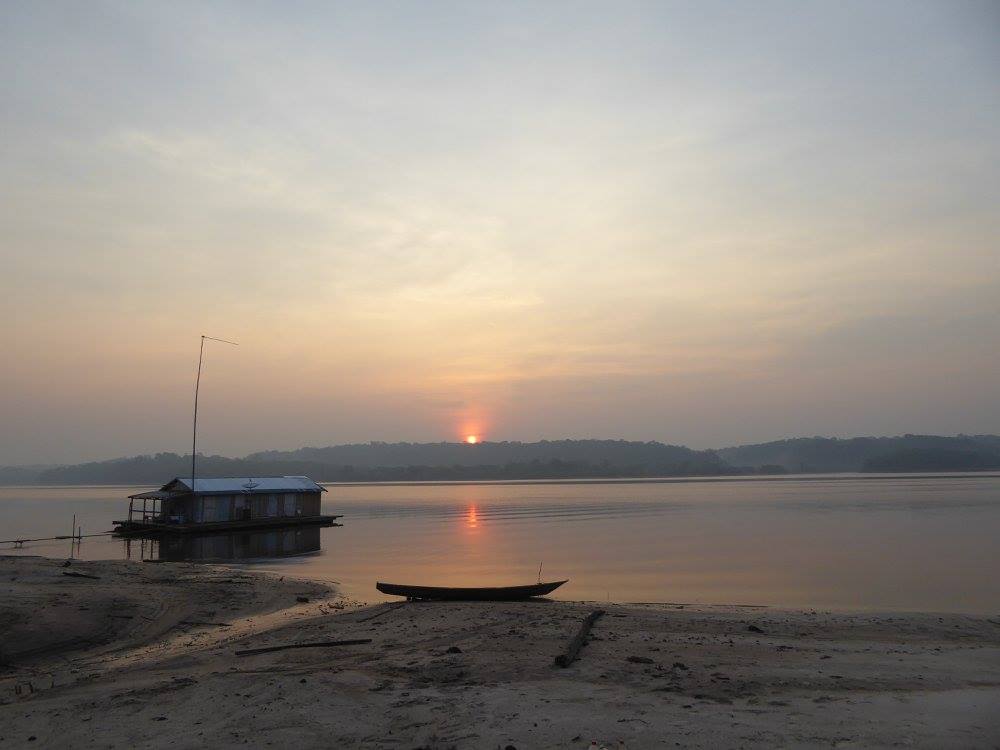
Sunrise on the Cuieras river, “Reserva do Cuieras”, close to Manaus, AM, Brazil.
Photo credit C.Ritter

Camila Ritter taking notes from field work.
Photo credit: N. Slobozian
2nd Global Soil Biodiversity
By Elizabeth Bach, Executive Director, Global Soil Biodiversity Initiative, Colorado State University
The 2nd Global Soil Biodiversity Conference (GSBC2) was held 15-18 October, 2017 in Nanjing, China. More than 1000 scientists from 47 countries gathered at the Nanjing International Youth Culture Centre to hear about the latest soil biodiversity science, network with colleagues new and old, and share new ideas.
Applying soil biodiversity science to global policy, Dr. Ronald Vargas, the Soils and Land Management Officer at the UN Food and Agricultural Organization and Secretary of the Global Soil Partnership, and Dr. Luca Montanarella, European Commission Joint Research Centre and chair of the Intergovernmental Technical Panel on Soils, called for a formal international assessment on soil biodiversity. There was much excitement around this call and it will be exciting to see it develop.
Conference co-chairs Prof. Ren-fang Shen (Institute of Soil Science, Chinese Academy of Science) and Prof. Yong-guan Zhu (Institute of Urban Environment, Chinese Academy of Science) shared recent developments in soil biodiversity research in China. Soil biology research has accelerated tremendously in the past 5 years in China and support for future work is strong. The China Soil Microbiome Initiative is a more than USD$35 Million project to systematically survey and sequence soil microbial diversity across China and link this biodiversity with key ecosystem services including nutrient cycling, crop production, and carbon storage. Leaders in the Soil Science Institute of the Chinese Academy of Science are seeking additional funding to extend support to include soil animals as well. In addition, the hundreds of Chinses graduate students, postdocs, lectures, and professors in attendance demonstrated deep knowledge, enthusiasm, and curiosity driving soil biodiversity research in China on topics ranging from agricultural production, ecosystem functioning, and restoration. In addition, the 19th National Congress of the Communist Party of China happened in Beijing the same week as GSBC2, and President Xi Jinping specifically included soil and ecological concerns as priorities for the Chinese agenda.
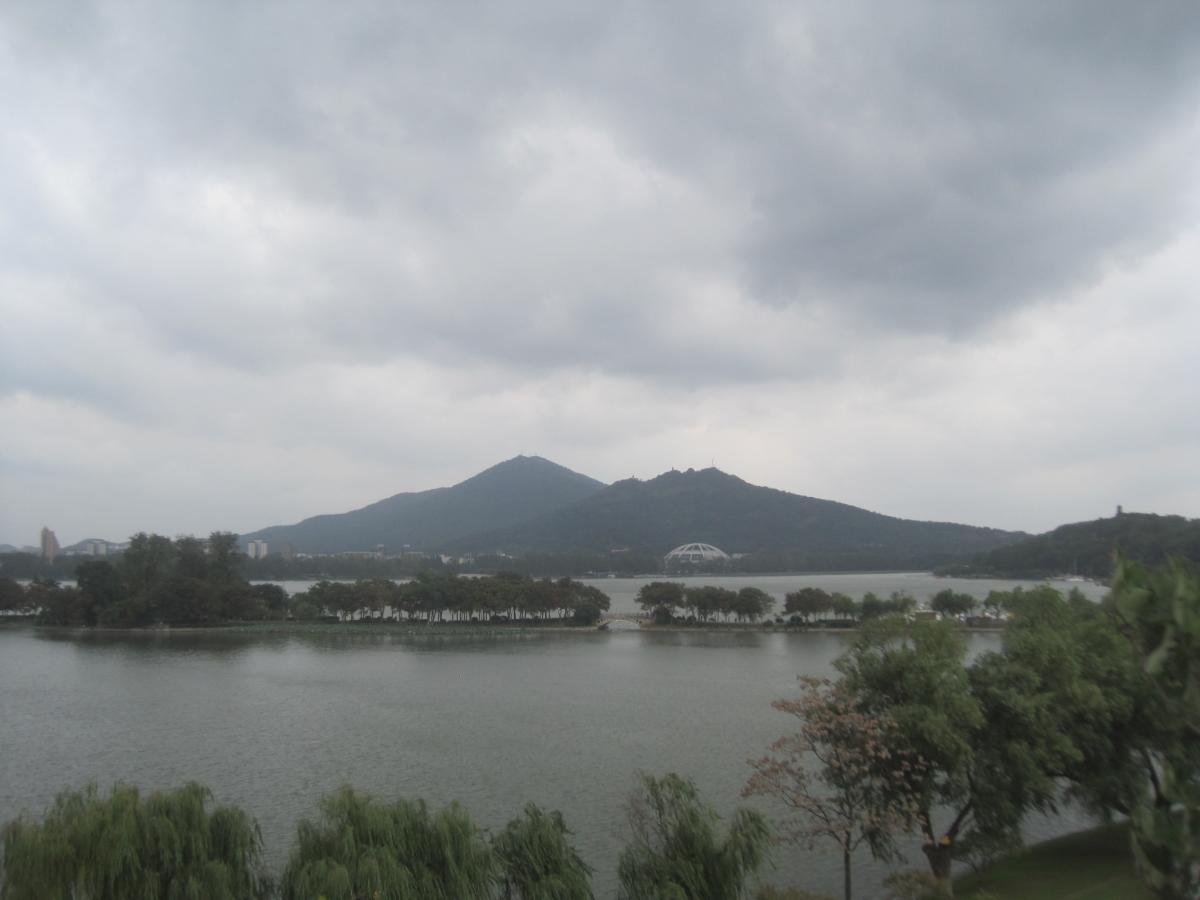
Zhongshan Mountain (Purple Mountain) is east of Nanjing, China.
Photo credit E.Bach
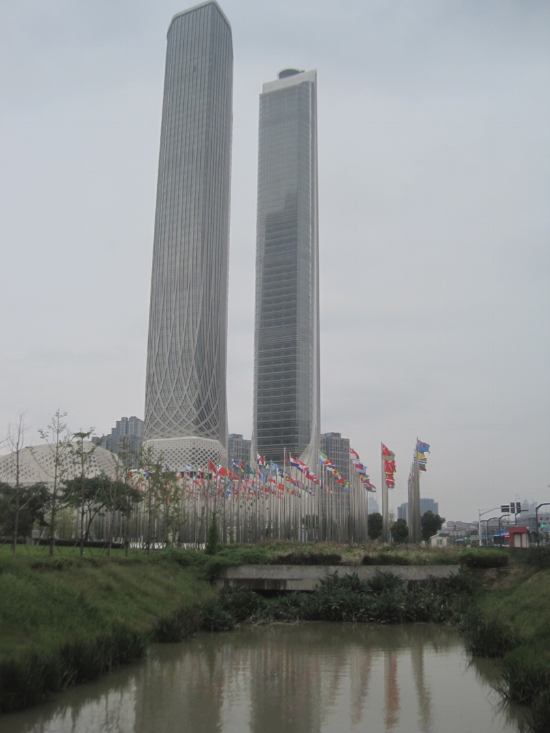
Nanjing International Youth Culture Centre
hosted GSBC2.
Photo credit E.Bach
Dr. Diana Wall, Scientific Chair for the Global Soil Biodiversity Initiative (Colorado State University), highlighted key Global Soil Biodiversity Initiative (GSBI) accomplishments since the 1st GSBC including publication of the Global Soil Biodiversity Atlas (including a new website), publication of many prominent papers, establishment and funding of working groups like sWORM, and incorporation of soil biodiversity into international policy documents including the Global Land Outlook (UNCCD), Global Assessment on Land Degradation and Restoration (Intergovernental Platform on Biodiversity & Ecosystem Services, IPBES, expected spring 2018), and Global Assessment on Soil Biodiversity (IPBES, expected spring 2018).
The GSBC2 featured research from around the world, including Europe, North America, South America (Brazil), Australia, and Africa. The European Joint Research Centre is gearing up for the 2018 Land Use/Land Cover Frame Survey (LUCAS) which will include DNA sequencing analysis for the first time. Dr. Brajesh Singh shared the first published results from the Biomes of Australian Soil Environments survey, showing distribution of bacteria and fungi across the nation. Brazilian scientists shared emerging work focused on soil microbes and fauna in the Amazonia region, investigating impacts of deforestation, agricultural management, and ecological restoration. Several Canadian and American scientists highlighted how soil biodiversity interfaces with global challenges including climate change, providing ecosystem services, ecological restoration success, and plant evolution.
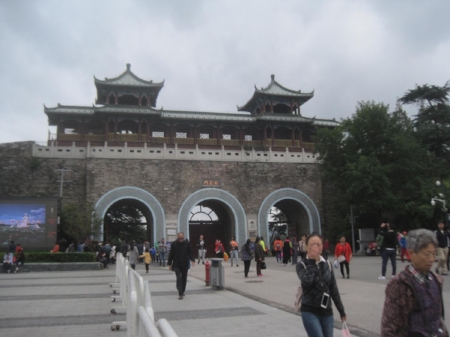
Xuanwu gate to the old Nanjing City Wall
Photo credit E.Bach
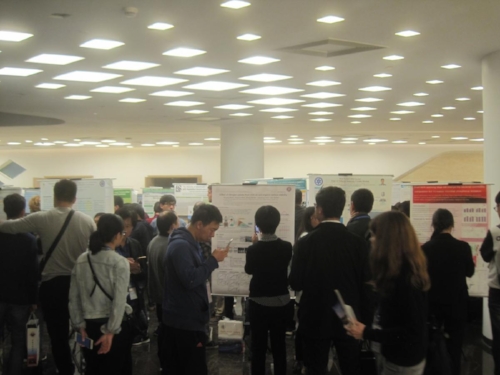
Participants enjoy a poster session at GSBC2.
Photo credit E.Bach
In addition to talks and posters, the conference featured several workshops and roundtables to share knowledge between established and early career scientists. Writing workshops were led by Dr. Wim van der Putten (Netherlands Institute for Ecology, NIOO-KNAW), Dr. Karl Ritz (University of Nottingham), and Dr. Josh Schimel (University of California Santa Barbara). In addition, there was an open evening social with the editors of Soil Biology & Biochemistry. Dr. Stefan Geisen (NIOO-KNAW) organized a roundtable featuring experts sharing best practices and emerging methods for studying soil organisms including bacteria, viruses, protists, nematodes, mites, molecular approaches for mesofauna, and working across disciplines and beyond the scientific world. Ting-wen Chen (University of Göttingen, Germany), Dr. Meixiang Gao (Harbin Normal University, China), Dr. Stefan Scheu (University of Göttingen, Germany), and Dr. Tancredi Caruso (Queen’s University of Belfast, Northern Ireland, UK) organized a roundtable focused on ecological theory and soil biota, which spurred exciting discussion late into the evening. Dr. Nadia Soudzilovskaia (Leiden University, Netherlands) and Dr. Gerlinde de Deyn (Wageningen University, Netherlands) organized a roundtable linking soil biodiversity to ecosystem functioning and provisioning of ecosystem services. These provided important opportunities for attendees to interact in focused small-groups and develop important career skills.
Look at the full program, including keynote abstracts here: http://ddl.escience.cn/f/PsCF
The 3rd Global Soil Biodiversity Conference will likely happen in 2020, stay tuned for more information!

Soil modeling for everyone: From concept to simulations
By Katherine Todd-Brown, USA @KatheMathBio

Computational and mathematical modeling are increasingly in demand as society tries to apply current scientific understanding to future soil management practices. The flux of carbon from the soil to atmosphere in particular is a major uncertainty of future climate projections. Soil carbon is also a critical component of soil health. In addition, many funding agencies are interested in coupling experimental and modeling approaches to better target scientific inquiry and extrapolate into murky futures.
Computational and mathematical models are generally thought of as tools for projecting into the future, but they can also help design and run experiments that might otherwise be costly or even impossible to carry out in the lab/field. You can turn off gravity in a model. While I say this with a bit of tongue in check, imagine directly exploring the effects of capillary action vs gravitational forces in soil wetting. Something that is completely impractical in the real world can become almost trivial in the computer.
Models are frequently seen as this magic box that, if you can just figure out how to plug your data in, will tell the rest of the world how critically important your research is. As a modeler, I’ve found that my colleagues who work primarily in the field and/or on the bench are frequently at a bit of a loss how to wave this magic wand. Fully characterizing a site to run an off-the-shelf model like DayCent can be overwhelming or just plain intractable depending on the location. Plus experimental treatments or particular measurements will often not have direct representation in these off-the-shelf models, precisely because their effects are novel or uncertain and thus of interest.
So where does that leave us?
Fortunately, if you design experiments and interoperate their results, you are most of the way there; even if you are a field or laboratory scientist who hasn’t written mathematical equation since your college math class. Numerical models are formalizations of conceptual frameworks that every scientists use on a daily basis. We tell stories of how we think the world works in our grant proposals and manuscripts. Those stories are models in their most basic forms; English, Mandarin, mathematics, and computer code are just a different languages that can be used to convey some scientific understanding to the broader world. By telling stories of how we think the world works, scientists are creating models.
The main difference between conceptual models and numerical models is precision. Human language is generally very fuzzy leaving quite a bit of room for interpretation to the listener. Mathematics, on the other hand, is extremely precise. It’s one thing to say that the change in soil carbon is the difference between the inputs and outputs, and another to state: . This mathematical formulation has several embedded assumptions in it like: soil carbon does not change with space, and inputs change over time but that the decay rate doesn’t. Mathematics does not allow you to sweep anything under the rug, instead you must explicitly state what your assumptions are and under what conditions those hold true. While you can be as precise with an English description of your conceptual framework, it can be challenging to attain the level of detail you get from a mathematical formalization. But underpinning all this is still your original conceptual understanding of the research system.
On a practical level how do you move from this conceptual framework to a precise mathematical formulation?
One way to do this is to collaborate with a mathematician or computer scientists. Be aware however that this will frequently require several conversations since you are likely talking with someone who has no soils training. The nutrient, parent material, and biological differences between a tropical oxisol and temperate molisol might be obvious to you but not to someone trained to locate bifurcation points in dynamical systems. Often times the different soil conditions will tie directly to different mathematical assumptions in ways that are not obvious at first glance. Lobbing your data over the discipline dividing wall won’t cut it. Instead, these collaborations require a lively and ongoing exchange.
Alternatively you can develop your own model. Frequently if you have a strong hypothesis driven experimental design, you can frame this hypothesis as a numerical model and probably already do on some level. Many statistical tests like linear regressions are, themselves, numerical models. A common problem with these statistical tests is that they assume normally distributed data and linear relationships, frequently not the case in soil systems. Diagramming the mass or energy path you are interested in will often lead to a set of differential equations. Once you have this mathematical formalization you can apply model-data integration techniques to fit descriptive parameters to your data.
By using numerical models informed by your scientific understanding you can dramatically increase the power of your statistical tests, compete different hypothesis, explore the relative importance of entwined mechanisms, and extrapolate findings into management scenarios. Models allow you to convey your scientific understanding, supported by your experimental data, with a precision that is difficult to achieve in a standard scientific narrative. While the end goal is scientific understanding not mathematical poetry, models are playing an increasingly important role in biogeochemistry.
Mathematics is the language of size, shape and order […] ~ Lancelot Hogben (1936)
Kathe Todd-Brown is a computational biogeochemist at the Pacific Northwest National Laboratory in Richland, Washington. She initially trained as a mathematician but it was a bit too clean. She transitioned to soil carbon cycling and couldn’t be happier to work in one of the most interesting systems on the planet.

An Experience with International Soil Research Networks
By Adam Cobb, Postdotoral Researcher, Oklahoma State Univeristy, USA
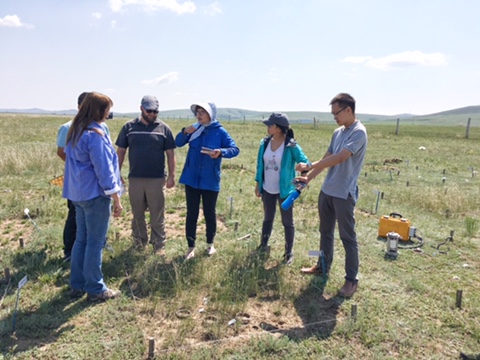
Collaborators discuss grassland soil carbon research near Hulanbuir, China. Photo credit Jiqiong Zhou
There is nothing quite like touching new soil. The soils of China are ancient, but this is my first chance to grab a handful. After leaving our hotel in Beijing at 4am, flying for three hours, and driving on a bombed-out road for another hour, we are in the steppe grasslands of Inner Mongolia in Northwest China.
We are here – with chestnut-colored soil in our hands – because of Jiqiong Zhou (soon to be Dr. Zhou) and her advisor, Dr. Yingjun Zhang. Sixteen months previously, Jiqiong (who also goes by Jolie) emailed Dr. Gail Wilson and asked if she could spend nine months with us at Oklahoma State University. Jiqiong’s research links above- and belowground influences on grasslands with particular emphasis on plant-microbial relationships, such as rhizobia/meliloti and arbuscular mycorrhizal symbioses, which is precisely Gail’s area of expertise.

Cattle grazing in the meadow steppe grasslands of Inner Mongolia, China. Photo credit Jiqiong Zhou
This PhD student exchange and research collaboration has been amazing. While Jolie was with us, she had the chance to visit the Konza Prairie Biological Research Station (NSF-LTER site) near Manhattan, Kansas, USA. We went up to establish grassland restoration plots, but took time to show her around the station, and particularly to see the bison. Later, she told us how lucky she thinks we are to research in such productive grasslands.
Back in China, her research grasslands are not as productive. With typically 300-400mm annual precipitation, they are a contrast to our tallgrass prairie systems. However, these semi-arid grasslands are critically important, not just for local sheepherders, but for soil ecologists. Climate models predict many mesic grasslands will become more arid during the 21st Century. It is crucial that we untangle the belowground drivers influencing aboveground productivity, plant species diversity, and ecosystem functions in semi-arid grasslands, if we are to manage our global grazing resources in a warmer and drier world.

Bison on Konza Prairie Biological Research Station near Manhattan, Kansas, USA. Photo credit Adam Cobb
This is where Jolie, and her colleagues in Dr. Zhang’s lab, conduct their valuable soil research. We walk across her plots, and see the yellow-flowered alfalfa (Medicago falcata) she established to rehabilitate these overgrazed areas. Belowground, she assessed how these reseeded legumes influence nutrient cycling, soil microbial communities, and soil metabolites. Today is a hot and sunny one, and we remark at how much data she has collected in these plots, often working by herself.
Jolie’s research is the combination of mechanistic assessments (e.g., microbial genomics) and applied questions. As part of the China Agricultural University’s College of Animal Science and Technology, she is keenly aware that these grasslands are provisioning ecosystems. Grazing treatments (real or simulated) are always part of the research design. Jolie is passionate about reseeded alfalfa because it can regenerate the landscape, increase incomes, and improve soil health.
Gail and I had an amazing experience with Jolie, Dr. Zhang, and their associates. We learned more about their culture, and we touched China’s soil. We are currently planning paired experiments assessing grassland plant and soil dynamics in both China and the USA. These collaborative research networks are key as we strive to conserve and restore global soils.

Biodiversity in a warmer world: lessons from soil nematodes
By Madhav Thakur, postdoctoral researcher, German Centre for Integrative Biodiversity Research (iDIV)

Predatory female nematode Clarkus sp. Image by M. Ciobanu
John Haldane, the famous evolutionary biologist, popularized the immense diversity of beetles by writing: “The creator, if he exists, has an inordinate fondness for beetles”. I wonder if Haldane was aware of nematodes. Nematodes are incredibly diverse and abundant tiny worms living almost everywhere on planet Earth. Some estimates point that we may have a million of nematode species on Earth. I remember Tom Bongers, a world-known nematode taxonomist, in his lectures saying every time one samples a forest soil, s/he is likely to find a new species of nematodes.
At the beginning of my PhD in 2013, I got interested in how on-going climate warming affects biodiversity. At this point, I already was familiar with the free-living nematodes in the soil, and in particular, impressed by their omnipresence in any environment. After the consultations with my PhD supervisor, Prof. Nico Eisenhauer, I decided to investigate whether warmer soil harbours less or more diversity of nematodes. Fortunately, I was offered to investigate nematode diversity in a long-term climate warming experiment in the meadows of Cedar Creek in Minnesota, USA. This climate warming experiment was unique for two reasons: 1) Climate warming was experimentally crossed with plant diversity and, 2) Plant diversity treatments in this experiment were the part of the BigBio experiment, which is one of the oldest biodiversity experiments in the world. Further, I was very excited to work with Prof. David Tilman, who is the principal investigator of this experiment, and well-known for his contributions for our understanding of the causes and consequences of biodiversity.

Aerial view of Biodiversity & Climate experiment. Image by J. Miller
Once I was able to collect nematodes and identify them with the help of colleagues (Dr. Marcel Ciobanu in particular), I started getting back at the warming and biodiversity question. Since we understand biodiversity in many different ways, I calculated many different metrics of biodiversity and see whether I could find any consistent pattern. The most striking and consistent pattern was that warming both increased and decreased nematode diversity. The key was whether the nematodes were from plant monoculture soils or from the soil of diverse plant communities. Warmer plant monocultures were lower in nematode diversity, whereas warmer diverse plant communities were higher in nematode diversity. Although these results were exciting, I did want to explore further. With the help of Dr. Oliver Purschke, I investigated whether warming also structures nematode communities in a given way. Indeed, the results revealed that nematodes were taxonomically more similar than expected in warmer soils independent of plant diversity. So even if warming increased nematode diversity in diverse plant communities, nematode communities become increasingly similar. We published these results recently in Science Advances.
The climate warming and biodiversity question will stay with ecologists for a longer time. Our results do provide some clues by using one of the most diverse and abundant organisms. At this stage, I am even more curious by the question how general are our results. Whether Haldane’s beetles, or our nematodes, biodiversity in a warmer world is very likely to be different than the past and present biodiversity.
Reference
M. P. Thakur, D. Tilman, O. Purschke, M. Ciobanu, J. Cowles, F. Isbell, P. D. Wragg, N. Eisenhauer (2017), Climate warming promotes species diversity, but with greater taxonomic redundancy, in complex environments. Science Advances 3, e1700866. Doi: 10.1126/sciadv.1700866.

Earthworm invasions in northern forests
By Erin Cameron, Postdoctoral Researcher, Helsinki University, Finland
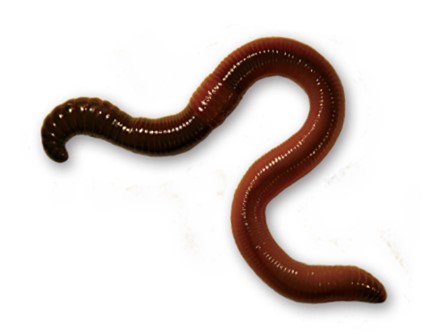
Lumbricus terrestris. Image by E. Cameron
Finishing my paper route always took longer on rainy days when I was a kid – I had to walk slowly to avoid stepping on earthworms and occasionally I stopped to move them off the sidewalk. I would never have believed that earthworms were invasive in much of Canada and the northern United States! In those previously glaciated areas, there are no native earthworms, but instead only European earthworms that were introduced to North America with the arrival of European settlers.
Earthworm populations can only expand about 5 to 15 meters per year on their own, and consequently people play a key role in their spread. For my master’s thesis with Dr. Erin Bayne at the University of Alberta, I tried to determine how earthworms were spreading in Alberta’s boreal forest. I was sold on the research question once I realized that I’d need to canoe or kayak across lakes to test whether earthworms were most common near boat launches where anglers might dump their earthworm bait. After a couple near misses but only one capsizing incident, we found that earthworms were present at approximately 70% of the boat launches and roads sampled, but only 35% of far shores and less than 15% of forest interiors. They were also more likely to occur at older roads than more recently built roads, suggesting that earthworms were introduced by vehicle traffic (their eggs can become stuck in tire treads) not during construction of the roads.
After examining how earthworms were being introduced, we started to investigate their effects in the boreal forest. Surprisingly to most people, earthworms do not always improve soil health or benefit other organisms. When exotic earthworms invade forests where there are no native earthworms, they consume leaf litter layers, mix organic and mineral soil horizons, and affect nutrient cycling. These impacts on soil structure and ecosystem functioning can then lead to cascading effects on other organisms. In northern Alberta, we found that earthworms decreased the thickness of the leaf litter layer, reduced the abundance and diversity of microarthropods, and decreased plant biomass, depending on the species. Not all species were negatively affected though – one of the key predators of earthworms, the American robin, was more likely to occur in areas where earthworms were present.
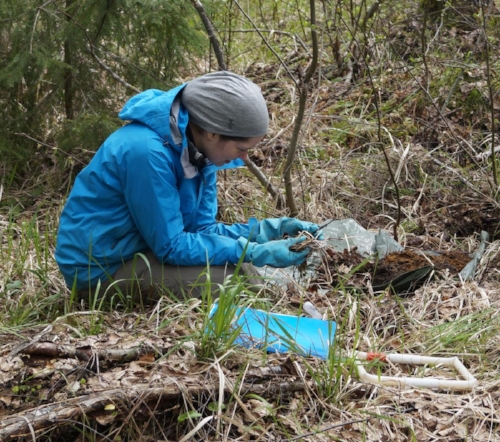
Sampling for earthworms in the boreal forest. Image by R. Rocha
Earthworm invasions are at an earlier stage in northern boreal forests than temperate hardwood forests, where the deep burrowing and mineral soil dwelling species that cause the largest changes are more widespread. At our study sites, the most common species is a litter dwelling species called Dendrobaena octaedra. But because most people are not aware that earthworms are invasive, they continue to introduce earthworms by dumping their bait, moving soil, or not cleaning their tires when travelling to remote areas. We started a citizen science project to collect data on earthworm distributions across Alberta, which at the same time serves to increase public awareness about earthworm invasions: http://worms.educ.ualberta.ca
However, earthworm invasions are occurring globally, rather than only in North America. We also lack data on distributions of native and exotic species of earthworms at broad scales, making it difficult to determine the key factors driving their distributions. To address this issue, we started a working group (sWORM; https://www.idiv.de/?id=429) at the German Centre for Integrative Biodiversity Research (iDiv) to synthesize data on earthworm distributions. Let us know if you have earthworm data and want to participate!
Further reading:
Cameron EK, Bayne EM, Clapperton MJ. 2007. Human-facilitated invasion of exotic earthworms into northern boreal forests. Ecoscience 14: 482-490.
Cameron EK, Bayne EM. 2012. Invasion by a non-native ecosystem engineer alters distribution of a native predator. Diversity and Distributions 18: 1190-1198.
Craven D et al. 2016. The unseen invaders: introduced earthworms as drivers of change in plant communities in North American forests (a meta-analysis). Global Change Biology 23: 1065-1074.

The Mysterious Case of the Microbe in the Soil
By Emm Fulk, graduate student, Rice University, Houston, TX, USA

Microbial biosensors sense and environmental signal and,
in response, produce a measurable reporter such as a gas.
Image by E. Fulk
Flagella? Check. Cell wall? Check. Cheesy music? Yes, that's right. What's a microbial detective without a melodramatic theme song?
Studies of soil microbiology have traditionally - and necessarily - been conducted from the outside in. Net fluxes of nutrients and gases from the soil environment can be chemically measured. High-throughput sequencing techniques can give metagenomic data, which provides a snapshot of the general composition of a soil microbiome. This is, essentially, a stakeout - we can get a general sense of a soil community by observing the surrounding environment and may be able to infer some activities by measuring who and what comes in and out. These strategies give us an overall picture of soil communities and their net interactions within the ecosystem but lack the spatial, temporal and chemical sensitivity to fully understand the internal dynamics of soil microbiomes.
We need a microbe on the inside.
The idea of using living microbes as biosensors is not especially new. To survive and adapt to new environmental stresses, such as nutrient or water deprivation, microbes have evolved networks to sense these changes and adapt their metabolism accordingly. Tying these naturally-evolved systems to a measurable reporter (for example, a fluorescent protein) is a logical step for understanding how microbes interact with their environment. Think of a light bulb and a light switch. The light switch senses whether it is on or off. The light bulb reports on the ON/OFF state of the light switch. Even if you can't see the switch, you can infer whether it is on or off by looking at the light bulb. Likewise, we can detect when a particular environmental condition elicits a microbial response by monitoring
the production of the reporter.
I know just the microbe for the job… he's sensitive, discreet and reports only to me.
For microbial biosensors to be useful in soil, their sensors and reporters must both be suitable for monitoring interesting
environmental conditions - for example, drought conditions, concentrations of nitrogen or carbon species, or cell-cell
communication signals. Sensors for -osmotic stress, nitrate, quorum sensing molecules and various heavy metals have been or are being
developed. These systems must also be sensitive to an environmentally relevant level of the signal. If too sensitive or not sensitive
enough, reporter production is not triggered at the right times to give useful information. Ideally, reporters need to be measurable in
situ. Traditional fluorescent or pigmented reports can't be used because, well, you can't see them in soil. Expanding our toolbox of
reporters would allow us to monitor cell growth as well as environmental response and to measure multiple signals.
The name's coli. Escherichia coli.

In standard biosensors without memory, microbes produce a reporter directly
in proportion to the level of signal. In biosensors with memory, the reporter is induced by the first instance of the environmental cue and remains on thereafter. The top cartoon shows how these two scenarios compare at the level of individual microbes. The bottom graph illustrates how reporter production differs at the whole-sample level. Image by E. Fulk
Even after engineering a useful biosensor, it remains to find suitable host microbe. Most synthetic biology is initially done in E. coli, because it is relatively well understood and easy to engineer. E. coli can also a good first organism to test biosensor function. Expanding our ability to engineer other microorganisms is a key challenge both for biosensors in soil ecology and for synthetic biology as a whole. Numerous other organisms - for example, several soil-dwelling Pseudomonas species - have successfully been engineered as biosensors. However expanding our repertoire of bacterial hosts will enable biosensors to be used in more microbial communities.
Where were the suspects on the night of the…high nitrate concentration?
Recent developments in synthetic biology have greatly expanded our ability to manipulate microbes and perform increasingly difficult computations. For example, microbes can now be programmed to produce a reporter only if both signal 1 AND signal 2 are present. Other logic functions (1 OR 2, 1 AND NOT 2, etc.) could allow for studying specific combinations of environmental conditions, such as in hot spots or during hot moments.
Cast in clay
By Max Helmberger, graduate student, New York State Agricultural Experiment Station, Geneva, New York, USA
Growing up an only child on a dirt road in the Northern Minnesota woods, I spent a lot of time outside, overturning the many thousands of glacier-strewn rocks around my house (at least the ones small enough to move) and gazing in awe at the centipedes, isopods, and invasive European earthworms underneath (which were promptly relocated to our compost bin). My first interest in soil in an academic context came the year after I graduated from high school, when I took a soil science course at my local community college. That class instilled in me a firm conviction that soil is humankind's most important natural resource, and clued me in to the fact that, in soil, there's far more than meets the eye.
After transferring to the University of Minnesota in Duluth to major in Biology, I took an entomology class and worked as a research assistant in an aboveground plant-insect ecology lab. I had always loved insects, arthropods, and invertebrates in general, and I greatly enjoyed the coursework and research experience, but wanted to connect it with my love of soil. I started searching Google Scholar for “soil arthropods”, and a few dozen soil ecology articles later, I was hooked, and I eventually sought out and accepted a M.S. position in the lab of Dr. Kyle Wickings at the New York State Agricultural Experiment Station, a satellite campus of Cornell University located in Geneva, New York. What I didn't know as I was reading all those papers, was that I would end up reporting all the knowledge I gained from them in a most unusual way.
Clay animation, for those unaware, is a form of stop-motion animation in which clay models are photographed, moved slightly, photographed again, and so on. The pictures are strung together and played in rapid succession to give the appearance of movement. Wallace and Gromit is arguably the most famous example of the medium. When I was 7 years old, my grandmother took me to an hour-long class in clay animation. I made a video of an anthropomorphic flower dancing to some sort of classical music riff. The VHS tape is certainly hiding somewhere in my house. Fast forward to my undergraduate entomology class, and I drew on those old memories for the course's final project to make a clay animation video on the life cycle of the gallmaking fly Eurosta solidaginis, the main study organism of my research advisors’ laboratory. The video was crude by my current standards, but got me a good grade in the class nevertheless.
At Cornell, where I'm currently working on my M.S. in Entomology, I’ve had the opportunity to draw from a unique funding source called the Extension/Outreach assistantship. Instead of working off a grant or being a teaching assistant (something difficult to do when based at a satellite research campus rather than the main university campus), I earned my stipend via progress on a variety of extension and outreach projects of my advisor's and my own devising. When applying for the assistantship and listing my project objectives, my advisor and some of the faculty members on the Extension/Outreach assistantship committee were skeptical until they saw the E. solidaginis video as a proof-of-concept, and in Spring semester of 2017, I was off to the races. To avoid some of the mistakes I made with my previous clay animation, I was very careful with how I went about planning and "filming" the videos. I wrote out all of my narration in advance as well a clear script of what specific actions I would portray. Then, I timed myself reciting the narration for each scene, and so could know in advance how many frames of animation I needed. This, combined with a nice DSLR camera as a Hanukkah present from my parents, would allow for much more cohesive and polished videos than my tale of the gallmaking fly. In the end, I produced three videos, Life Cycle of Entomopathogenic Nematodes, The Soil Food Web, and Ecosystem Services in Agriculture (though the latter includes some functions performed by aboveground organisms). My funding next semester will be from the same Extension/Outreach assistantship, so I plan to produce at least one more video in addition to my other projects, possibly two. From start to finish (writing the script, creating the models, creating the set, taking the photographs, editing the video, and recording the narration), each video took me between 15 and 20 hours to make. Each video consists of 350-400 individual images, with some being repeated here and there. They’ve been received well in the department, and the entomopathogenic nematode video has even been incorporated into several extension talks. The rest of the videos have ben showcased in a few classroom settings, and I am hoping to further expand their reach. I plan to make at least two additional videos in the fall, as I will again be funded through an Extension/Outreach assistantship.
My ultimate goal is that these videos provide an accessible way of communicating soil ecology and biodiversity to lay audiences, especially young ones. Despite being the prototypical "science nerd" growing up, and being an avid consumer of books, documentaries, and Web resources about the natural world, many of the soil animals I read about during my first forays into the primary literature were completely unknown to me. I had no idea there were mites beyond dust mites and the various parasitic taxa, and certainly didn't know there were any mites as cute as a galumnid oribatid. I had never even heard of diplurans, symphylans, pauropods, and some of the other more obscure soil organisms. I knew what a pseudoscorpion was, but didn’t know I could find them in the peat bog less than a mile from my house. And that rubbed me the wrong way. It's hard for young people to learn about the marvels of soil biodiversity, especially on their own. I know that 7 year-old Max would have gotten much more out of these videos than from one about a dancing flower, and he would have started playing around with Tullgren funnels much earlier than junior year of college. As such, if you enjoy my videos, I encourage you to share them however and wherever you like. They are available online as a YouTube playlist.
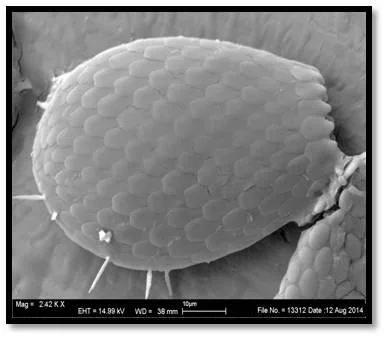
Soil protistology: a rising star?!
By: Valentyna Krashevska1, Stefan Geisen2
1Post-doc University of Goettingen, Germany
2Post-doc Netherlands Institute of Ecology, the Netherlands
Part 4 in our 4 part soil protist series

Image: Testate amoebae Euglypha
Soil protistology, despite a long history, is a rather unexplored field with many things to be studied. In the last three blogs we pointed out several of those points including unknown, yet huge diversity and abundance and the fundamental functional importance of protists in the soil food web and for plant growth promotion. They also are highly promising bioindicators to assess soil quality and allow palaeological reconstructions; for the latter, especially testate amoebae, which often have a rigid shell, play a key role.
At PROTIST 2016, around 200 protistologists are gathering, yet, less than 10 % of the participants work in soils. This is surprising taken into account that even editors of general ecological or soil journals are increasingly understanding the potential in the field of soil protistology; just in the last 12 months, three papers purely focusing on soil protists (nematode feeding protists, huge diversity of parasitic protists in soilsand parasitic protists in soil animals) were in the spotlight and received highlight articles (1, 2, 3, respectively). Many recent studies found their place in the highest (ecological) journals and this trend is likely to continue.
Now it is the time to actually jump on that train and bring this understudied field to the next level; many exciting discoveries are awaiting to be made, which might well outweigh findings on the other, better studied microbial groups of bacteria and fungi. This especially counts for integrating soil protist work with work on other soil organisms and in more general ecological studies!
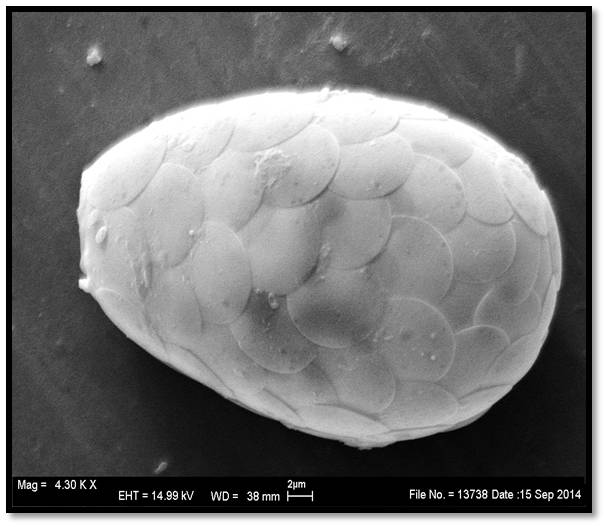
Testate amoebae Tracheleuglypha
Protists, the overseen guardians of soil microbiome function
By Assistant Professor Dr. Alexandre Jousset, Utrecht University, The Netherlands
This is part 3 in a 4 part blog series on soil protists.
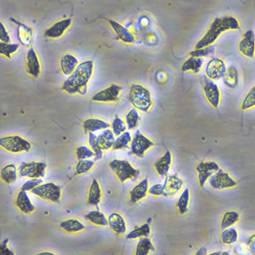
Cercomonas sp., a bacterivorous amoebae.
Soil microbes provide essential functions supporting soil fertility and plant health. Recent advances in sequencing technologies have favored a boom in studies investigating soil microbiome diversity and function. However, to date most studies have focused on bacteria and fungi, neglecting other trophic levels. This focus may be very convenient, as many functional genes are now described. It however oversees the function of predators as regulators of microbial communities.
Soil bacterial and fungal communities are typically top-down controlled. In other words, the main selective pressure is predation, not resource availability. The main predators of bacteria are protists and nematodes. These organisms, albeit unrelated, have been historically grouped as “microfauna”, reflecting that protist have been mostly investigated by zoologists and botanists, not by microbiologists. This discipline separation has contributed to neglecting protists in environmental microbiology. With these lines I aim at bridging these two research fields.
Protists can affect bacterial communities and soil fertility in several ways: By massively consuming bacteria, they release the nutrients contained in their preys, accelerating nutrient cycling. This increased nutrient availability can stimulate plant growth as well as nitrification process. Further, by reducing bacterial biomass, they alleviate competition and allow for more synergies between competing species. Protists are further very selective and will ingest only specific preys. They select preys based on their morphology, surface properties and toxicity. This selection has a strong impact on microbial functions linked to soil fertility. For instance, bacteria producing large amounts of exopolysaccharides may be better protected. These compounds play an important role in gluing soil particles together. We can thus expect that protozoa predation may improve soil structure. A range of studies have also revealed the functional overlap between antibiotics linked to disease suppression and protozoa inhibition. Several bacteria can naturally protect plants against disease by producing antibiotics and are seen as a promising alternative to pesticides. However, most attempts to use these bacteria in natural soil have failed. They either die out or evolve to lose their plant protective ability. Protists are here the guardians that “force” bacteria to produce antibiotics. They eat up bacteria lacking antibiotics, creating more space for the well-defended – and coincidentally plant protecting ones. Previous experiments in my group have shown that adding bacterivorous amoebae to soil can increase the success of plant-beneficial microbes by a factor three. In addition, bacterivorous protists are sensed by bacteria, that upregulate antibiotics production as a defense mechanism. These different protists-bacteria interactions can have a profound effects on soil fertility. We could for instance show that addition of bacterivorous protists could induce soil suppressiveness against the fungal pathogen Fusarium oxysporum. First commercial application of protozoa are already on the market and help for instance mineralize organic fertilizers and promote plant growth in sustainable agriculture.
I conclude that protozoa should be included in further microbiome studies and green biotechnology strategies aiming at reducing fertilizer and pesticide use in the agriculture.
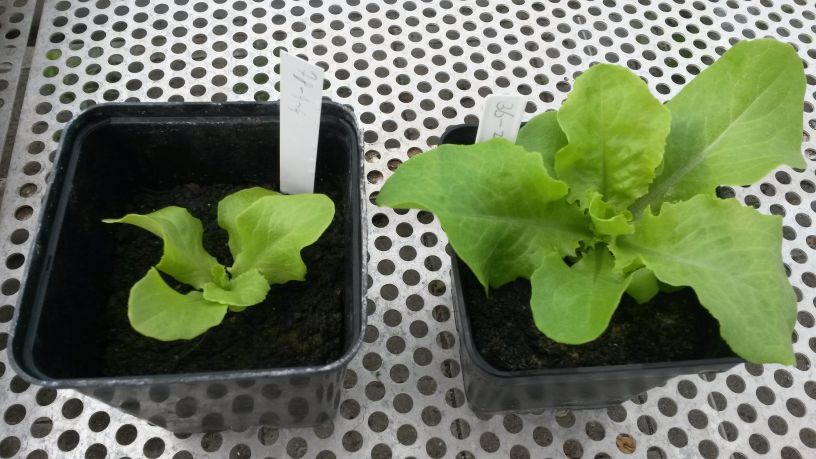
Lettuce grown on compost, left without addition of protists, right with addition of Cercomonas sp.

The Many Roles of Protists in the Soil
By Dr. Enrique Lara, University of Neuchâtel, Switzerland
This is part two in four part soil protist series! Part 1 can be read here.

Figure 1: This unidentified amoeba is one of the members of the extremely diverse protist community inhabiting the soil of a common indoor flower pot; new species can be found even in the least exotic environments! This species feeds on yeasts and bacteria.
Protists are extremely diverse in soils, often reaching thousands of species of protists and fungi per gram. If we bring these numbers to our scale of perception, this means that a little piece of soil the size of a fingernail hosts a number of species comparable to the diversity of insects in a hectare of tropical rainforest! Like in the jungle, the different organisms play various roles in the soil ecosystem. Globally, these roles can be divided in three great categories: osmotrophs, phototrophs and phagotrophs.
Osmotrophs absorb their food from the environment; they are unable to engulf preys. They play a fundamental role in the decomposition of dead organic matter produced by plants. Mostly fungi take this role, but they are not alone! Another very common group of soil osmotrophs is the oomycetes, which closely resemble fungi but are now classified within the stramenopiles- a group very distant to fungi together with many algae such as the marine kelps! Some organisms evolved from photosynthetic ancestors to live in the absence of light and became secondarily osmotrophs, like the green alga Polytomella. Osmotrophic organisms often tend to become parasites during evolution; they start the evolutionary process as mostly free-living organisms that infect occasionally any potentially weakened host. Then, they become gradually more and more specialized and virulent. Many species of fungi and oomycetes are well known plant parasites, and are responsible for huge economic losses every year. Others infect animals (including humans) and even other fungi! Other groups are entirely parasitic such as the Phytomyxea (plant parasites) and the Apicomplexans (animal parasites, including amongst others the agent of malaria Plasmodium falciparum), which can be extremely abundant and diverse in soils. However, osmotrophs can also become Mr. Niceguy and collaborate with plants: mycorrhiza are the most widespread and famous example.
Being a phototroph, obtaining energy from the sun like a plant, in soils may seem contradictory; however, phototrophic organisms are numerous and diverse as well. Logically, they are limited to the upper part of the soil that is reached by light; they are responsible (together with mosses and cyanobacteria) for the formation of so-called cryptogamic crusts, which are common in deserts and high altitude soils. Some of these groups are well known in lakes and rivers (like diatoms, green algae, xanthophytes), but most often species are specific to soils as they went through specific adaptations to be able to colonize these environments.
Many protists in soils are phagotrophic, which means that they prey on other organisms through phagocytosis (just like the macrophages of our immune system). Bacteria are a common food source for them, and it has been shown that predation by protists is the main source of mortality for soil bacteria. By eating these preys, nutrients are released and taken up by plants; it has been shown that this phenomenon, coined the soil microbial loop, is key in driving plant productivity. However, all bacteria are not equally preyed upon by protists, and food preferences vary drastically even between closely related protist species. On the other hand, bacteria are by no means defenceless and produce secondary metabolites that can kill protist predators. This make trophic interactions between protists and bacteria extremely complex. But bacteria are by no means the only prey of protists. Fungi are also consumed, and some species of ciliates possess a cytostome (=cell mouth) that prevents them from eating anything else; they are simply unable to consume bacteria! Others are top predators and will feed only on other protists. Some, like the tiny shelled amoeba Cryptodifflugia, are able to kill even nematodes, and practice a kind of pack hunting to slay their victims which weigh about hundred times more than them!

Figure 2: A testate amoeba, Centropyxis aerophila, hunting for small protists and fungi in its favourite environments, forest litter. It uses its pseudopod to move forward and capture preys by immobilizing them before engulfing.
The situation is complicated even more as some organisms may belong to two functional categories at the same time. Many soil flagellates and amoebae are capable of both actively hunting for preys and absorbing nutrients from the environment, thus combining phagotrophy and osmotrophy. Phototrophy and phagotrophy are also often combined, especially in wet soils like in peatlands (where it is largely practised by golden alga like Ochromonas, Synura and Mallomonas). Altogether, functional diversity of eukaryotes in soils is immense. Our knowledge on their diversity is now at a turning point where it starts to be evaluated, but still remains an open field for new, exciting discoveries.