

Blog Archive:
Beneath Our Feet

Soil Carbon Modelling with Soil Fauna and Humus Forms
By Cindy H. Shaw, Oleg Chertov, and Darrell Hoffman*

An example of a mull humus form.
Image by D.Hoffman
Soil fauna are key agents in different types of organic debris processing in the forest floor and mineral topsoil, resulting in humus forms. The humus form that develops at any given site is the result of the amounts and types of litter inputs (such as wood, leaves, roots) from local vegetation, temperature and moisture conditions, and the dynamics of soil biota including fauna, fungi, and bacteria. Humus forms are most broadly divided into three orders: mor, moder, and mull. Each order is associated with a set of physical properties that are easily observed and are related to processes occurring in the forest floor and the underlying mineral soil.

An example of a moder humus form.
Image by C.McNalty
Mors are characterized by a distinct boundary between organic and mineral soil horizons, often with plentiful plant roots and fungal hyphae throughout the organic layers. Mulls develop when there is sufficient mixing of organic and mineral soil often resulting from the activities of soil fauna; they have a relatively thick, dark, mineral Ah horizon enriched with organic matter.
Moders are humus forms with properties that transition between those of mors and mulls. The orders can be further divided into groups described by horizon types (such as L, F, H, Ah), which indicate the stage of decomposition, or include descriptors for composition (such as woody, fungal mossy).
The activities of different organisms and the interactions among them have direct consequences for carbon dynamics, as they are the agents driving rates of mineralization and respiration, as well as stabilization, and sequestration. Although the actions of soil fauna mediate the cycling and storage of carbon, the direct effects of these organisms can be difficult to study, and until now have not been included in carbon models. In addition, most carbon models focus on predicting carbon emissions because of the great interest in greenhouse gases, and they neglect the formation and storage of soil organic matter, which is important in carbon sequestration.

An example of a fungal mor humus form.
Image by C.McNalty

An example of a woody mor humus form.
Image by C.McNalty
Recently, a model developed by scientists in Russia, Germany and Canada, Romul_Hum (the soil module of the individual tree forest growth model EFIMOD), integrates knowledge of humus form development, soil fauna food webs, dynamics of fungi and bacteria, and the resultant formation and stabilization of carbon in soil organic matter. Romul_Hum accounts for the many belowground interactions (fungivory, bactivory, predator-prey relationships) between soil fauna, bacteria, and fungi and how these interactions are regulated by the qualities of incoming vegetative material. Unlike other models, which treat decomposers as a homogenous group, Romul_Hum uses variations in the ratios of fungal to bacterial biomass, and the ratios of carbon to nitrogen in the fungal and bacterial biomass. Based on published soil fauna data, different types of food webs are defined for combinations of decomposers and types of horizons in humus forms. An earthworm module was developed with parameters for for food palatability, ingestion and egestion, food consumption, lifespan, excretion, and assimilation efficiency. It is especially important to understand the effects of earthworms interacting with other soil fauna activities in Canada as earthworms are invasive to Canada’s large boreal forest (see blog: Earthworm invasions in northern forests). As earthworms spread through the Canadian boreal forest, they will change the carbon dynamics and carbon balance of the ecosystems.

An invasive earthworm and lepidoptera larva in a boreal forest soil sample.
Image by C.McNalty
Romul_Hum could be used to predict, understand, and quantify those changes. The types of changes to the forest carbon cycle from invasive earthworms is dependent on the species of earthworm(s) present. These changes can include mixing organic material in the forest floor with the mineral soil below, shifting the balance between fungal and bacterial biomass, and stabilizing carbon in soil organic matter as it moves through the gut of the earthworm, or as earthworms ingest and stabilize faeces produced by meso-fauna. Beyond these effects, earthworms can change the food and habitat available for other groups of soil fauna, such as nematodes, mites, and springtails, affecting the survival and success of meso-faunal populations.

The Forest Floor Recovery Index
Image by D.Hoffman
By acknowledging and accounting for the complex interactions between soil faunal food webs and their habitat (humus forms), the modelling approach of Romul_Hum provides a means to evaluate how management, and potentially climate change, affects relationships between soil fauna biodiversity and soil carbon sequestration. In Europe, humus form classification is currently being refined within the HUMUSICA project. In Canada, humus forms are used as part of a system (Forest Floor Recovery Index) to evaluate the success of reclamation after mining.
*Cindy Shaw (cindy.shaw@canada.ca(link sends e-mail)) is a Research Scientist, and Darrell Hoffman (darrell.hoffman@canada.ca(link sends e-mail)) is a Forest Soil Research Assistant, for the Canadian Forest Service at Natural Resources Canada. Oleg Chertov is a scientist who has worked in Russia, Germany, and Finland, and created the Romul_Hum models with Alex Komarov

Romul_Hum predictions of soil carbon stocks and their distribution between the mineral Ah and organic O horizons, depending on presence of mesofauna and
earthworms.
Image by O.Chertov

Building mud castles: A perspective from brick laying termites
By Nikita Zachariah, Graduate Student, Centre for Ecological Science, Indian Institute of Science, Bengaluru, India

Termite mound construction using bricks.
Image by N. Zachariah
Walking in the wild or even in a metro city like Bengaluru you are sure to find animal homes in all their grandeur — bower bird nests, bee hives, spider webs and termite mounds. These aesthetically designed structures have always fascinated architects, naturalists and laypersons alike, yet we barely know how they are built — what are the basic building blocks or bricks in these constructions and how materials are chosen for these constructions.
In consultation with my PhD advisors Prof. Renee M. Borges and Prof. Tejas G. Murthy I decided to explore the physical, chemical and behavioural aspects of one such construction — the termite mound. Though made up of soil, termite mounds can stand in sun and rain for decades together without dissolving thanks to termite secretions that are mixed with soil during construction imparting ten fold increase to its strength. Termite mounds can house more than a million termite individuals and can reach a height of 10 metres. At a human scale this would correspond to a building 10 kilometres tall… taller than Mount Everest!! Termites construct these mounds without an architect, without a masterplan, in fact without even seeing the structure they are building. Yes, these termites are blind. Not only do termites engineer their mounds, they also engineer entire ecosystems making them drought resistant. Yet, little do we know about the basic building blocks of these mounds and what makes a geographic region conducive for mound construction.
I studied Odontotermes obesus species of termites in Bengaluru, India. It is widely distributed in the Indian subcontinent and makes mounds that are upto 2.5 meters tall. It aggregates moist soil particles into tiny balls which act as bricks during mound construction. The different castes of termites (such as major and minor termites) make different sizes of bricks which they jointly pack like golf balls in a jar with marbles filling the space between the balls thereby achieving tight packing and consequently high strength. Moreover, in the lab they were even able to use materials like glass beads for making bricks. Since termites used a totally unfamiliar material, glass beads, I was curious to know what else can they handle? In order to understand this I gave them every material I could get my hands on — metal powders, jellies, even tissue paper and paraffin wax!! To my surprise they used all the materials as long as they were able to walk and chew on them. But they do had their personal favourites, e.g. they loved granular materials over others and were equally willing to use non-familiar materials like glass beads as the familiar ones (soil). Other properties that determined the ease of handling were hydrophilic, osmotically inactive and nonhygroscopic nature, surface roughness, rigidity and presence of organic matter. These material properties along with the availability of moisture and favourable climatic conditions will determine the global geographic distribution of termites, a matter of considerable importance given their roles as ecosystem engineers. This study also takes us towards understanding how tiny termites make mounds that any engineer would envy.

Bricks made by different castes of termites.
Photo credit: N. Zachariah

Packing of large and small bricks during construction.
Photo credit: N. Zachariah
The study was published in the journal Scientific Reports (https://www.nature.com/articles/s41598-017-04295-3) and was featured in Science magazine (http://www.sciencemag.org/news/2017/07/thesetermites-can-use-glass-beads-build-mounds).
Lab webpage: Prof. Renee M. Borges (http://ces.iisc.ernet.in/renee/), Prof. Tejas G. Murthy (http://civil.iisc.ac.in/~tejas/)

Earthworm invasions in northern forests
By Erin Cameron, Postdoctoral Researcher, Helsinki University, Finland
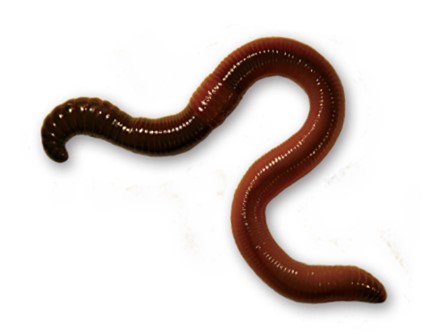
Lumbricus terrestris. Image by E. Cameron
Finishing my paper route always took longer on rainy days when I was a kid – I had to walk slowly to avoid stepping on earthworms and occasionally I stopped to move them off the sidewalk. I would never have believed that earthworms were invasive in much of Canada and the northern United States! In those previously glaciated areas, there are no native earthworms, but instead only European earthworms that were introduced to North America with the arrival of European settlers.
Earthworm populations can only expand about 5 to 15 meters per year on their own, and consequently people play a key role in their spread. For my master’s thesis with Dr. Erin Bayne at the University of Alberta, I tried to determine how earthworms were spreading in Alberta’s boreal forest. I was sold on the research question once I realized that I’d need to canoe or kayak across lakes to test whether earthworms were most common near boat launches where anglers might dump their earthworm bait. After a couple near misses but only one capsizing incident, we found that earthworms were present at approximately 70% of the boat launches and roads sampled, but only 35% of far shores and less than 15% of forest interiors. They were also more likely to occur at older roads than more recently built roads, suggesting that earthworms were introduced by vehicle traffic (their eggs can become stuck in tire treads) not during construction of the roads.
After examining how earthworms were being introduced, we started to investigate their effects in the boreal forest. Surprisingly to most people, earthworms do not always improve soil health or benefit other organisms. When exotic earthworms invade forests where there are no native earthworms, they consume leaf litter layers, mix organic and mineral soil horizons, and affect nutrient cycling. These impacts on soil structure and ecosystem functioning can then lead to cascading effects on other organisms. In northern Alberta, we found that earthworms decreased the thickness of the leaf litter layer, reduced the abundance and diversity of microarthropods, and decreased plant biomass, depending on the species. Not all species were negatively affected though – one of the key predators of earthworms, the American robin, was more likely to occur in areas where earthworms were present.
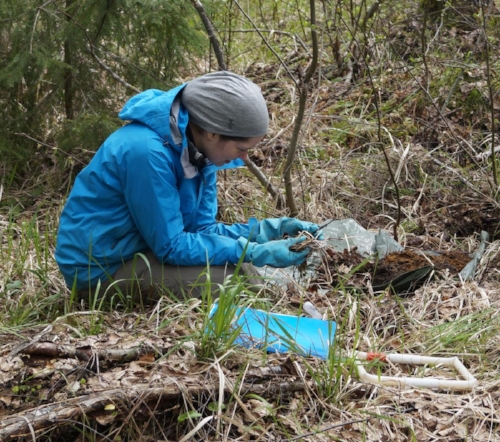
Sampling for earthworms in the boreal forest. Image by R. Rocha
Earthworm invasions are at an earlier stage in northern boreal forests than temperate hardwood forests, where the deep burrowing and mineral soil dwelling species that cause the largest changes are more widespread. At our study sites, the most common species is a litter dwelling species called Dendrobaena octaedra. But because most people are not aware that earthworms are invasive, they continue to introduce earthworms by dumping their bait, moving soil, or not cleaning their tires when travelling to remote areas. We started a citizen science project to collect data on earthworm distributions across Alberta, which at the same time serves to increase public awareness about earthworm invasions: http://worms.educ.ualberta.ca
However, earthworm invasions are occurring globally, rather than only in North America. We also lack data on distributions of native and exotic species of earthworms at broad scales, making it difficult to determine the key factors driving their distributions. To address this issue, we started a working group (sWORM; https://www.idiv.de/?id=429) at the German Centre for Integrative Biodiversity Research (iDiv) to synthesize data on earthworm distributions. Let us know if you have earthworm data and want to participate!
Further reading:
Cameron EK, Bayne EM, Clapperton MJ. 2007. Human-facilitated invasion of exotic earthworms into northern boreal forests. Ecoscience 14: 482-490.
Cameron EK, Bayne EM. 2012. Invasion by a non-native ecosystem engineer alters distribution of a native predator. Diversity and Distributions 18: 1190-1198.
Craven D et al. 2016. The unseen invaders: introduced earthworms as drivers of change in plant communities in North American forests (a meta-analysis). Global Change Biology 23: 1065-1074.

The Mysterious Case of the Microbe in the Soil
By Emm Fulk, graduate student, Rice University, Houston, TX, USA

Microbial biosensors sense and environmental signal and,
in response, produce a measurable reporter such as a gas.
Image by E. Fulk
Flagella? Check. Cell wall? Check. Cheesy music? Yes, that's right. What's a microbial detective without a melodramatic theme song?
Studies of soil microbiology have traditionally - and necessarily - been conducted from the outside in. Net fluxes of nutrients and gases from the soil environment can be chemically measured. High-throughput sequencing techniques can give metagenomic data, which provides a snapshot of the general composition of a soil microbiome. This is, essentially, a stakeout - we can get a general sense of a soil community by observing the surrounding environment and may be able to infer some activities by measuring who and what comes in and out. These strategies give us an overall picture of soil communities and their net interactions within the ecosystem but lack the spatial, temporal and chemical sensitivity to fully understand the internal dynamics of soil microbiomes.
We need a microbe on the inside.
The idea of using living microbes as biosensors is not especially new. To survive and adapt to new environmental stresses, such as nutrient or water deprivation, microbes have evolved networks to sense these changes and adapt their metabolism accordingly. Tying these naturally-evolved systems to a measurable reporter (for example, a fluorescent protein) is a logical step for understanding how microbes interact with their environment. Think of a light bulb and a light switch. The light switch senses whether it is on or off. The light bulb reports on the ON/OFF state of the light switch. Even if you can't see the switch, you can infer whether it is on or off by looking at the light bulb. Likewise, we can detect when a particular environmental condition elicits a microbial response by monitoring
the production of the reporter.
I know just the microbe for the job… he's sensitive, discreet and reports only to me.
For microbial biosensors to be useful in soil, their sensors and reporters must both be suitable for monitoring interesting
environmental conditions - for example, drought conditions, concentrations of nitrogen or carbon species, or cell-cell
communication signals. Sensors for -osmotic stress, nitrate, quorum sensing molecules and various heavy metals have been or are being
developed. These systems must also be sensitive to an environmentally relevant level of the signal. If too sensitive or not sensitive
enough, reporter production is not triggered at the right times to give useful information. Ideally, reporters need to be measurable in
situ. Traditional fluorescent or pigmented reports can't be used because, well, you can't see them in soil. Expanding our toolbox of
reporters would allow us to monitor cell growth as well as environmental response and to measure multiple signals.
The name's coli. Escherichia coli.

In standard biosensors without memory, microbes produce a reporter directly
in proportion to the level of signal. In biosensors with memory, the reporter is induced by the first instance of the environmental cue and remains on thereafter. The top cartoon shows how these two scenarios compare at the level of individual microbes. The bottom graph illustrates how reporter production differs at the whole-sample level. Image by E. Fulk
Even after engineering a useful biosensor, it remains to find suitable host microbe. Most synthetic biology is initially done in E. coli, because it is relatively well understood and easy to engineer. E. coli can also a good first organism to test biosensor function. Expanding our ability to engineer other microorganisms is a key challenge both for biosensors in soil ecology and for synthetic biology as a whole. Numerous other organisms - for example, several soil-dwelling Pseudomonas species - have successfully been engineered as biosensors. However expanding our repertoire of bacterial hosts will enable biosensors to be used in more microbial communities.
Where were the suspects on the night of the…high nitrate concentration?
Recent developments in synthetic biology have greatly expanded our ability to manipulate microbes and perform increasingly difficult computations. For example, microbes can now be programmed to produce a reporter only if both signal 1 AND signal 2 are present. Other logic functions (1 OR 2, 1 AND NOT 2, etc.) could allow for studying specific combinations of environmental conditions, such as in hot spots or during hot moments.

Urban Expansion, Land Cover, and Soil Ecosystem Services
By Ciro Gardi, Scientific Officer, Animal & Plant Health Unit, European Food Safety Authority, Parma, Italy

We are aware, especially the readers of this blog, of the immeasurable value of soil and of its unique and essential role. The focus of the Global Soil Biodiversity Initiative is the variety of living forms that soil can host, and it is clear that in order to have soil biodiversity we need to have soil. In other words, we will not be able to protect soil biodiversity if we are not protecting the soil as whole. Unfortunately, there are several processes leading to soil degradation and the intensity and combination of them vary across the globe.
One of the most irreversible process, often overlooked, is represented by soil sealing, consequent the expansion of urban and industrial areas or the construction of transport infrastructures. The intensity of this process can be extremely high, especially in the countries with fast economic and/or demographic growth, and often it occurs at the expenses of the most valuable and fertile soils. After the soil is sealed, due to the construction of buildings, roads, etc., all the soil ecosystem services are lost or severely compromised. Not only to the capacity of soil to be used for agriculture, but also its capability to infiltrate water, to store carbon, etc.
A newly published book, Urban Expansion, Land Cover and Soil Ecosystem Services, is an accurate overview of the impact of urban expansion processes on the provision of soil ecosystem services. From the analysis of the magnitude and intensity of these processes at global scale, to the assessment of the impact of soil sealing and land take on the capability of soil to produce food and biomass. The role of soil in agricultural production is probably the most obvious: according to FAO, 95% of our food derive directly or indirectly from soil, and by to 2050 we will need to increase the food production by 70%. There are however other soil ecosystem services essential for human wellbeing, and more in general for the protection of life on the Earth. The regulation of water cycle and most terrestrial biogeochemical cycles rely on soil. The existences of the majority of terrestrial ecosystems also depend on soil.
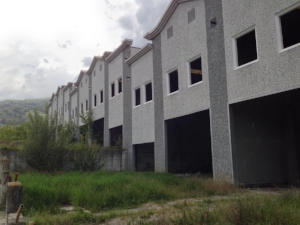
Often new residential, commercial or industrial buildings are realised only for speculative reasons and remain unused for ever. Photo credit: Ciro Gardi

Soil sealing prevents, or strongly compromise all soil ecosystem functions. This is an example of an exception: the vigour of this plant is able to break the asphalt coverage sealing the soil. Photo credit: Ciro Gardi

An example of a construction site. Soil is subject to several types of
degradation processes: compaction,contamination and finally sealing.
Photo credit: Ciro Gardi
It is essential then to have a more responsible use and planning of this strategic and pivotal non-renewable resource, sharing our knowledge of its values and role, with policy makers, land use and urban planners, but also citizens. In Europe, a public campaign has been recently launched (People4Soil - https://www.people4soil.eu/en ) to request the declaration of a soil protection Directive at the EU level. This is an example of the efforts of awareness raising that made possible to spread among citizens the comprehension of the role of soil, as essential element of the natural capital.
Learn more about the book here:
Cast in clay
By Max Helmberger, graduate student, New York State Agricultural Experiment Station, Geneva, New York, USA
Growing up an only child on a dirt road in the Northern Minnesota woods, I spent a lot of time outside, overturning the many thousands of glacier-strewn rocks around my house (at least the ones small enough to move) and gazing in awe at the centipedes, isopods, and invasive European earthworms underneath (which were promptly relocated to our compost bin). My first interest in soil in an academic context came the year after I graduated from high school, when I took a soil science course at my local community college. That class instilled in me a firm conviction that soil is humankind's most important natural resource, and clued me in to the fact that, in soil, there's far more than meets the eye.
After transferring to the University of Minnesota in Duluth to major in Biology, I took an entomology class and worked as a research assistant in an aboveground plant-insect ecology lab. I had always loved insects, arthropods, and invertebrates in general, and I greatly enjoyed the coursework and research experience, but wanted to connect it with my love of soil. I started searching Google Scholar for “soil arthropods”, and a few dozen soil ecology articles later, I was hooked, and I eventually sought out and accepted a M.S. position in the lab of Dr. Kyle Wickings at the New York State Agricultural Experiment Station, a satellite campus of Cornell University located in Geneva, New York. What I didn't know as I was reading all those papers, was that I would end up reporting all the knowledge I gained from them in a most unusual way.
Clay animation, for those unaware, is a form of stop-motion animation in which clay models are photographed, moved slightly, photographed again, and so on. The pictures are strung together and played in rapid succession to give the appearance of movement. Wallace and Gromit is arguably the most famous example of the medium. When I was 7 years old, my grandmother took me to an hour-long class in clay animation. I made a video of an anthropomorphic flower dancing to some sort of classical music riff. The VHS tape is certainly hiding somewhere in my house. Fast forward to my undergraduate entomology class, and I drew on those old memories for the course's final project to make a clay animation video on the life cycle of the gallmaking fly Eurosta solidaginis, the main study organism of my research advisors’ laboratory. The video was crude by my current standards, but got me a good grade in the class nevertheless.
At Cornell, where I'm currently working on my M.S. in Entomology, I’ve had the opportunity to draw from a unique funding source called the Extension/Outreach assistantship. Instead of working off a grant or being a teaching assistant (something difficult to do when based at a satellite research campus rather than the main university campus), I earned my stipend via progress on a variety of extension and outreach projects of my advisor's and my own devising. When applying for the assistantship and listing my project objectives, my advisor and some of the faculty members on the Extension/Outreach assistantship committee were skeptical until they saw the E. solidaginis video as a proof-of-concept, and in Spring semester of 2017, I was off to the races. To avoid some of the mistakes I made with my previous clay animation, I was very careful with how I went about planning and "filming" the videos. I wrote out all of my narration in advance as well a clear script of what specific actions I would portray. Then, I timed myself reciting the narration for each scene, and so could know in advance how many frames of animation I needed. This, combined with a nice DSLR camera as a Hanukkah present from my parents, would allow for much more cohesive and polished videos than my tale of the gallmaking fly. In the end, I produced three videos, Life Cycle of Entomopathogenic Nematodes, The Soil Food Web, and Ecosystem Services in Agriculture (though the latter includes some functions performed by aboveground organisms). My funding next semester will be from the same Extension/Outreach assistantship, so I plan to produce at least one more video in addition to my other projects, possibly two. From start to finish (writing the script, creating the models, creating the set, taking the photographs, editing the video, and recording the narration), each video took me between 15 and 20 hours to make. Each video consists of 350-400 individual images, with some being repeated here and there. They’ve been received well in the department, and the entomopathogenic nematode video has even been incorporated into several extension talks. The rest of the videos have ben showcased in a few classroom settings, and I am hoping to further expand their reach. I plan to make at least two additional videos in the fall, as I will again be funded through an Extension/Outreach assistantship.
My ultimate goal is that these videos provide an accessible way of communicating soil ecology and biodiversity to lay audiences, especially young ones. Despite being the prototypical "science nerd" growing up, and being an avid consumer of books, documentaries, and Web resources about the natural world, many of the soil animals I read about during my first forays into the primary literature were completely unknown to me. I had no idea there were mites beyond dust mites and the various parasitic taxa, and certainly didn't know there were any mites as cute as a galumnid oribatid. I had never even heard of diplurans, symphylans, pauropods, and some of the other more obscure soil organisms. I knew what a pseudoscorpion was, but didn’t know I could find them in the peat bog less than a mile from my house. And that rubbed me the wrong way. It's hard for young people to learn about the marvels of soil biodiversity, especially on their own. I know that 7 year-old Max would have gotten much more out of these videos than from one about a dancing flower, and he would have started playing around with Tullgren funnels much earlier than junior year of college. As such, if you enjoy my videos, I encourage you to share them however and wherever you like. They are available online as a YouTube playlist.

What lies beneath: South Africa’s megadiversity of soil biota Part I
By Dr. Charlene Janion-Scheepers, Postdoctoral Research Fellow, Monash University, Australia
This is the first in a three-part blog series highlighting the rich soil biodiversity found in South Africa.

Soils are integral to agricultural productivity, biodiversity and the maintenance of ecosystem services. However, soil ecosystem research depends on foundational biological knowledge that is often missing. In a recent review published in Pedobiologia, we review the current knowledge on the soil biota of South Africa. The paper outlines the literature and sampling methods used to assess soil biota, the available taxonomic expertise and depository of main collections within South Africa, the availability of identification guides and online resources, and the status and distribution of described species.
This review was the result of two workshops held by the Soil Ecosystem Research Group in South Africa (SERG). We are a soil biodiversity research group that provides a platform for linking and promoting research on soil organisms. One of the first priorities identified by SERG was the need to collate and mobilise data and collections such that we can consolidate and compare the state of knowledge of each group. We also identified that foundational work on soil organisms is needed to facilitate research on soil health, as was outlined in our paper The unknown world: Understanding soil health in South Africa.

The first Soil Health Workshop held at the XVII Entomological Society of Southern Africa Congress in Bloemfontein, 6 July 2011.
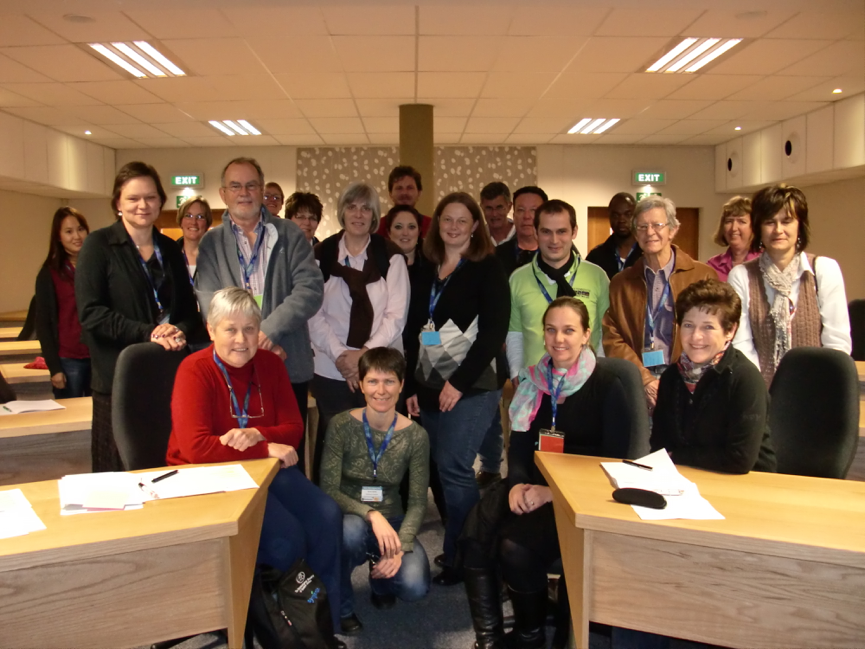
Second workshop of the Soil Ecosystem Research Group held at the XVIII Entomological Society of Southern Africa Congress, 2 July 2013, North West University, Potchefstroom.
In our next blog What lies beneath: South Africa’s megadiversity of soil biota (part II) we will discuss the rich soil biodiversity found in South Africa.